


Washingtonia filifera, California palm
Howard, Janet L. 1992. Washingtonia filifera, California palm. In: Fire Effects Information System, [Online]. U.S. Department of Agriculture, Forest Service, Rocky Mountain Research Station, Fire Sciences Laboratory (Producer). Available: https://research.fs.usda.gov/feis/species-reviews/wasfil
| Abbreviation | Common Name | Scientific Name | Classification | Status |
|---|---|---|---|---|
| Plants | ||||
| WASFIL | California palm | Washingtonia filifera | Life Form: Plants/Tree Kingdom: Plantae Class: Monocot Order: Arecales Family: Arecaceae Genus: Washingtonia | Fed. Protected: No Nativity: Native Invasiveness: Noninvasive |


Taxonomy
The scientific name of California palm is Washingtonia filifera (Linden) Wendl. [3,24,28].
Synonyms
- Washingtonia robusta Wendl.
- Washingtonia arizonica Cook
Other Common Names
California fan palm, Washington palm, California Washington-palm, desert palm
General Distribution
California palm occurs in disjunct groves from the Turtle and Cottonwood Mountains and the Twenty-nine Palms region of the Mojave Desert, California south to the Sierra de Juarez, the Sierra San Pedro Martir, and Sierra Pinnate Mountains, Baja California [27,39]. Four groves are located in Clark County, Nevada [7], and five others are in La Paz and Yavapai Counties, Arizona [23]. Most United States populations occur within the Colorado Desert along the San Andreas Fault. Due to California palm's value as an indicator species (see Site Characteristics), all known California palm communities have been mapped [7]. It is extensively planted as an ornamental in semiarid and subtropical regions of the world [9], and has naturalized in some places [24].
States
- United States: AZ CA HI NV
- Mexico
Site Characteristics
Topography and soils: California palm occurs at elevations below 3,500 feet (1,067 m) [24]. It serves as an indicator species, denoting sources of year-round surface water in desert [22,33]; it is found near seeps, springs, and streams [33]. It also occurs in canyons where water is channeled from nearby mountains, in alluvial fan edges where groundwater is trapped by bedrock, and where water percolates through rock fractures caused by earthquake faulting [32]. Soils are generally undeveloped and low in organic matter except in densely vegetated oases. Hillside oases soils consist of lacustrine sediments of mud and rock, while wash oases soils also contain sand. Seep oases have fine, flocculent soils and are frequently covered by a thin crust of salts, which tends to minimize soil erosion. If such soils are thickly crusted, undergrowth is sparse or absent. Most soils supporting California palm are high in pH (average pH 9.2) [40]. Soils in its root zone, however, are generally less alkaline than topsoils [33].
Climate: California palm grows in a semiarid climate. Temperatures are typically hot in summer (average 107 degrees Fahrenheit [42 deg C]) and below freezing in winter. Temperature extremes recorded near one Colorado Desert oasis are 13 and 125 degrees Fahrenheit (-17 and 52 deg C). Oases temperatures are generally more moderate than the open desert, being cooler in summer and warmer in winter. Average annual precipitation ranges from 3 inches (8 cm) at the lowest to 8 inches (20 cm) at the highest elevations of California palm's range. Most precipitation falls from December to March, but locally beneficial rains occur from July through September. Lightning is common during such storms [40].
Plant Communities
California palm forms open to dense groves in moist areas, often providing 100 percent of overstory cover [34]. Understory species are sparse in dense groves and more alkaline areas; they may be abundant in open groves or favorable sites [15]. California palm communities separate into three distinct zones: the hydric zone, the oasis-proper, and the oasis-desert ecotone. Oases located at wash or stream sites gradually intergrade into open desert, while oases in seep areas generally have abrupt ecotones, grading sharply into xeric desert communities such as mesquite (Prosopis spp.) [40]. Publications naming California palm as a dominant species are as follows:
- Sonora Desert [5]
- Natural terrestrial communities of California [15]
- Riparian forest and scrubland community types of Arizona and New Mexico [34]
- The vascular plant communities of California [35]
Plant associates: Overstory associates not listed in table A1 include Fremont cottonwood (Populus fremontii), saltcedar, paloverde (Cercidium floridum), and California sycamore (Plantus racemosa) [7,30,40]. Understory associates include cattail (Typha spp.), reed (Phragmites australis), cane (Arundinaria spp.), Olney bulrush (Scirpus olneyi), Torrey seepweed (Suaeda torreyana), desert willow (Salix gooddingii), arrowweed (Pluchea sericea), saltgrass (Distichlis spp.), mesquite, alkali sacaton (Sporobolus airoides), alkali goldenbush (Haplopappus acradenius), desert holly (Atriplex hymenelytra), and allscale saltbush (A. polycarpa) [1,7,24,30,40].
Botanical Description

A California palm stand in Anza-Borrego Desert State Park, San Diego County, California. (CC BY-NC 4.0)
California palm is a native evergreen monocot from 30 to 50 feet (9-15 m) in height and 1 to 2 feet (0.3-0.6 m) in diameter. The crown is a rosette of large leaves. It is supported by a columnar trunk. Unburned trunks are covered by a mass of pendent dead leaves called a shag or skirt. Outer trunk tissue consists of a thick, barklike rind. The inflorescence is a spadix. The fruit is a drupe containing a single large seed [28,32,33]. California palm is a phreatophtye [40]. Roots are variously described in the literature as shallow [1] or deep [28]. Presumably, root depth varies with depth of the water table, with palms growing near seeps and springs having the more shallow root systems. Determining the exact age of palms is difficult because tree-ring counts cannot be made on monocots. The maximum age attained by this species is estimated to be 200 years. Mature trees typically live about 150 years [40]. California palm can withstand about 22 hours of subfreezing temperature [9].
Raunkiaer Life Form (Raunkiaer 1934)
- Phanerophyte
Seasonal Development
Flowering occurs in May and June [32]. The leaves die at the end of the summer growing season, remaining attached to the trunk [33]. Fruits ripen in September [23], and seeds ripen and drop from November to January [19,6].
Regeneration Processes
California palm regenerates from seed [12]; vegetative reproduction does not occur (J. W. Cornett, in [22]). Cultivated trees have flowered at age 19 [26], but the age at which trees growing under natural conditions first flower is unreported. Pollination is predominantly insect-mediated (J. W. Cornett, in [22]), but self-pollination may also occur [22]. Natural populations of California palm are reseeding well [23]. A heavy crop for an individual tree probably approaches 10,000 fruits. In the southern Anza-Borrego region of California, 11 percent of trees fruited 1 year, followed by 57 to 59 percent of trees fruiting in the following 3 years [6]. Seeds are disseminated primarily by the coyote [7,40]. Because of its fruit-eating habit and broad range of travel between water sources, coyote often transport seeds over considerable distances [32]. The four California palm groves of southern Nevada probably established from seed in coyote scat [7]. A comparison of seed collected from the ground surface and seed collected from coyote scat showed that the pericarp was missing from 94 percent of coyote-consumed seed. Removal of the pericarp increases the probability of germination. Sixty-three percent of coyote-consumed seed tested in this study germinated, as compared to 34 percent of that in the control group [8]. Seed in coyote scat are rarely consumed by passing animals [7]. Gray fox also consume and disseminate seed. Birds generally consume only the fruit, not the seed [32]. The western and mountain bluebird and the cedar waxwing, however, eat both fruit and seed, disseminating the seed in droppings. Seed in bird droppings are usually disseminated within or close by the grove of the parent tree. The seed appears to be difficult for these birds to digest, and are often regurgitated. Regurgitated seed may still be partially covered by fruit fragments, which reduces germination rates. Rodent predation of seed in bird droppings or vomit is high [6]. Seed remains viable in seedbanks for up to 6 years [19]. Germination is hypogeal [36]. Seedlings require a moist mineral seedbed and partial shade to full sun. They cannot establish on highly alkaline soils [39]. Seedling recruitment frequently occurs in a flush during wet years [40].
California palm fruit allelopathically inhibits germination and growth of other species under laboratory conditions [7].
Successional Status
California palm is moderately shade tolerant when young, becoming intolerant with age [28,40]. California palm communities require moist pioneer conditions [40]. They are invaded by shrubs in the absence of fire, creating environmental conditions which eventually kill the palms [1,40]. (see Fire Management Considerations and Other Management Considerations).
Immediate Fire Effects

These long, flammable shags reach from bole base to the crown. The tree on the right shows evidence of past fire, with a charred trunk and a short, charred shag.
The immediate effect of fire on an individual California palm varies according to the tree's fire history. Fire causes the greatest reduction of outer vascular bundles with the initial burning of the highly flammable shag [40]. Typically, all dead leaves are burned as well as most of the living rosette of leaves [32]. The trunk may be repeatedly burned as leaves in the crown detach and slide down the trunk, ringing the base with fresh fuel. Subsequent fires burn lesser amounts of the trunk because the shag, previously removed by fire, requires a number of years to regain thickness and length. Each subsequent fire further chars the trunk surface, increasing fire resistance [40]. No data are available on the effects of fire on seedlings. Vogl [40] believes seedlings require a fire-free period of a few years before fire resistance is attained.
Postfire Regeneration Strategy (Stickney 1989)
- Tree without adventitious-bud root crown
- Secondary colonizer - on-site seed
- Secondary colonizer - off-site seed
Fire Adaptations
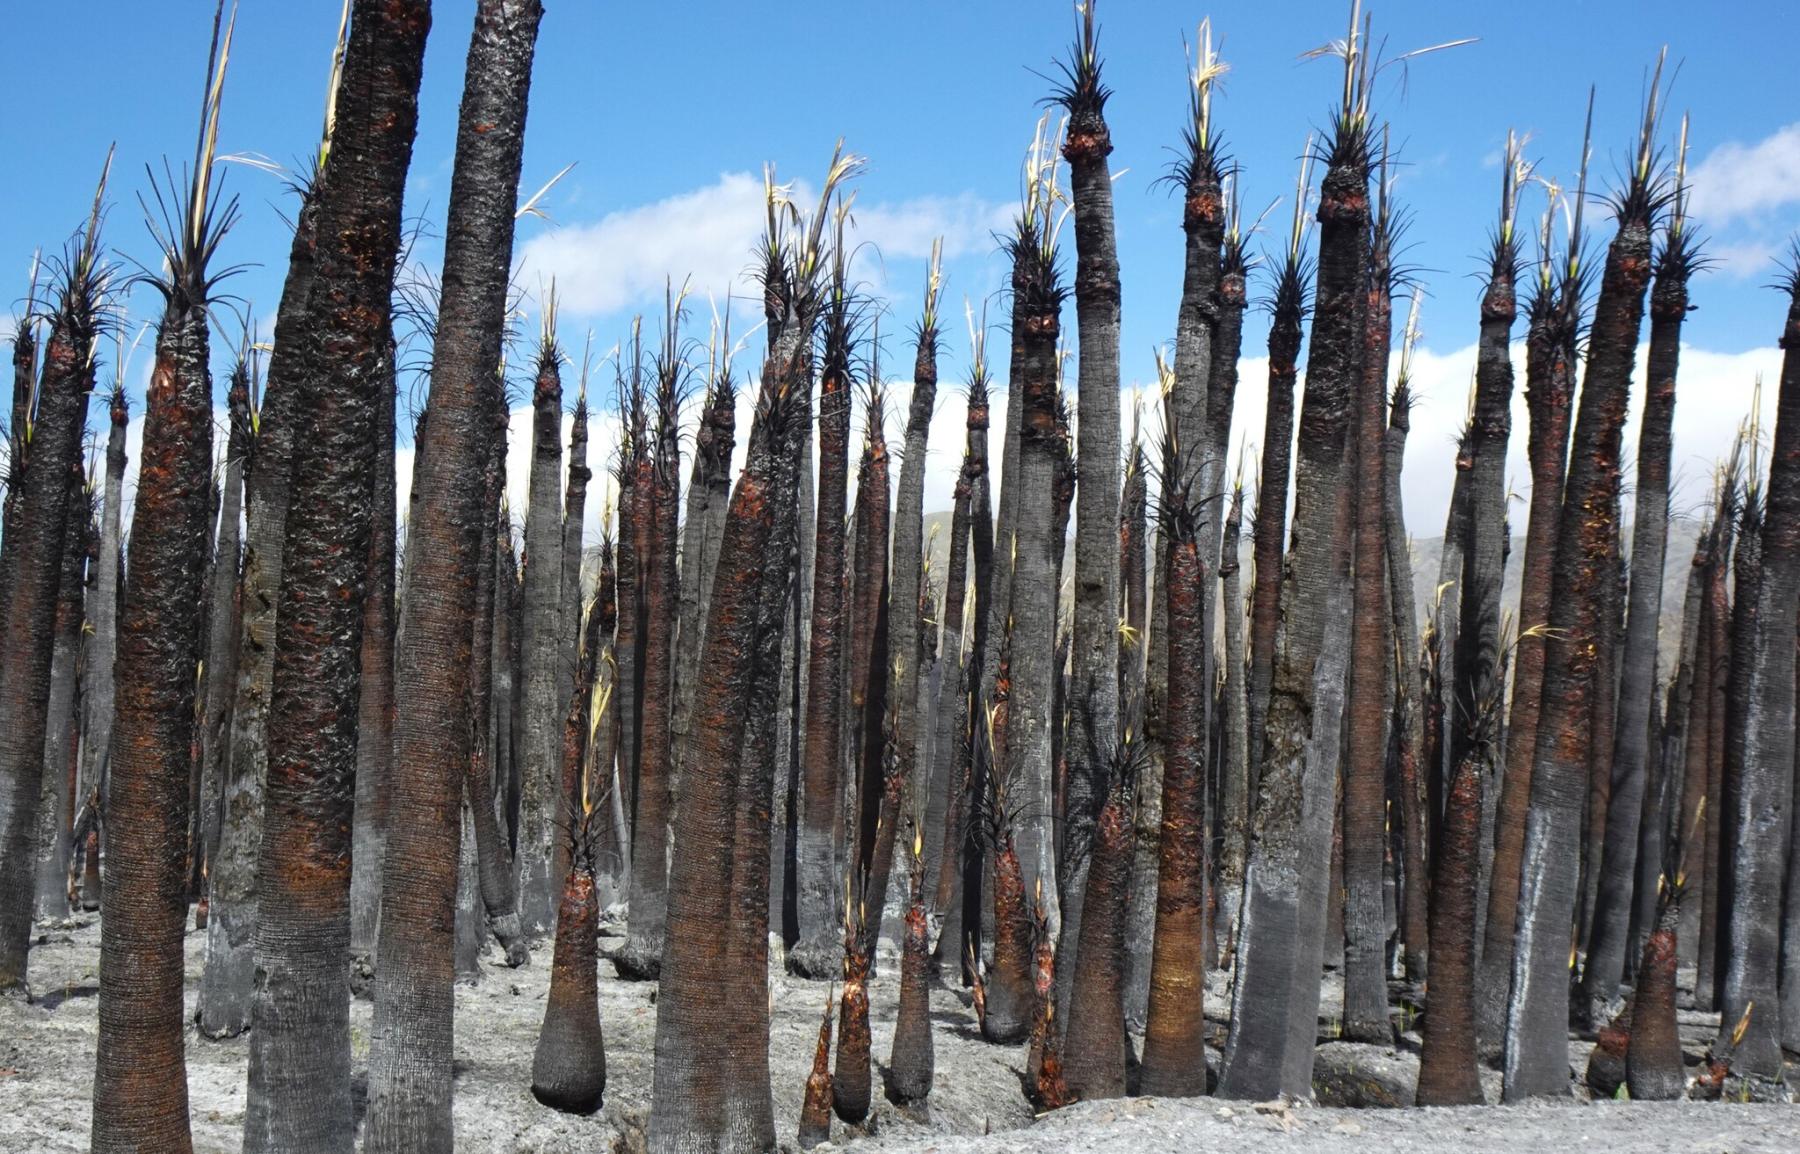
California palms are fire resistant. They are rarely killed by either the initial burning of their shag or by subsequent burnings. Burning experiments show that their fibrous trunks are difficult to ignite and almost impossible to flame. Each successive burning kills some outer vascular bundles and burns off some of the trunk, causing a reduction of trunk diameter. Crown fire, a common occurrence, reduces crown size. Repeated burnings sometimes results in fire-dwarfed trees. Reduction in trunk and crown reduces the evapotranspiration rate, making more effective use of limited water supplies and allowing for a greater number of palms per oasis. Wind-blown, advancing crown fire does not inflict as much damage or kill as many palms as a slow-moving fire burning in still air [40].
Plant Response to Fire
Fire releases saplings suppressed by the shade of shrubs. Young palms, freed from competition for water and sunlight, grow vigorously in fire-opened sites [40].
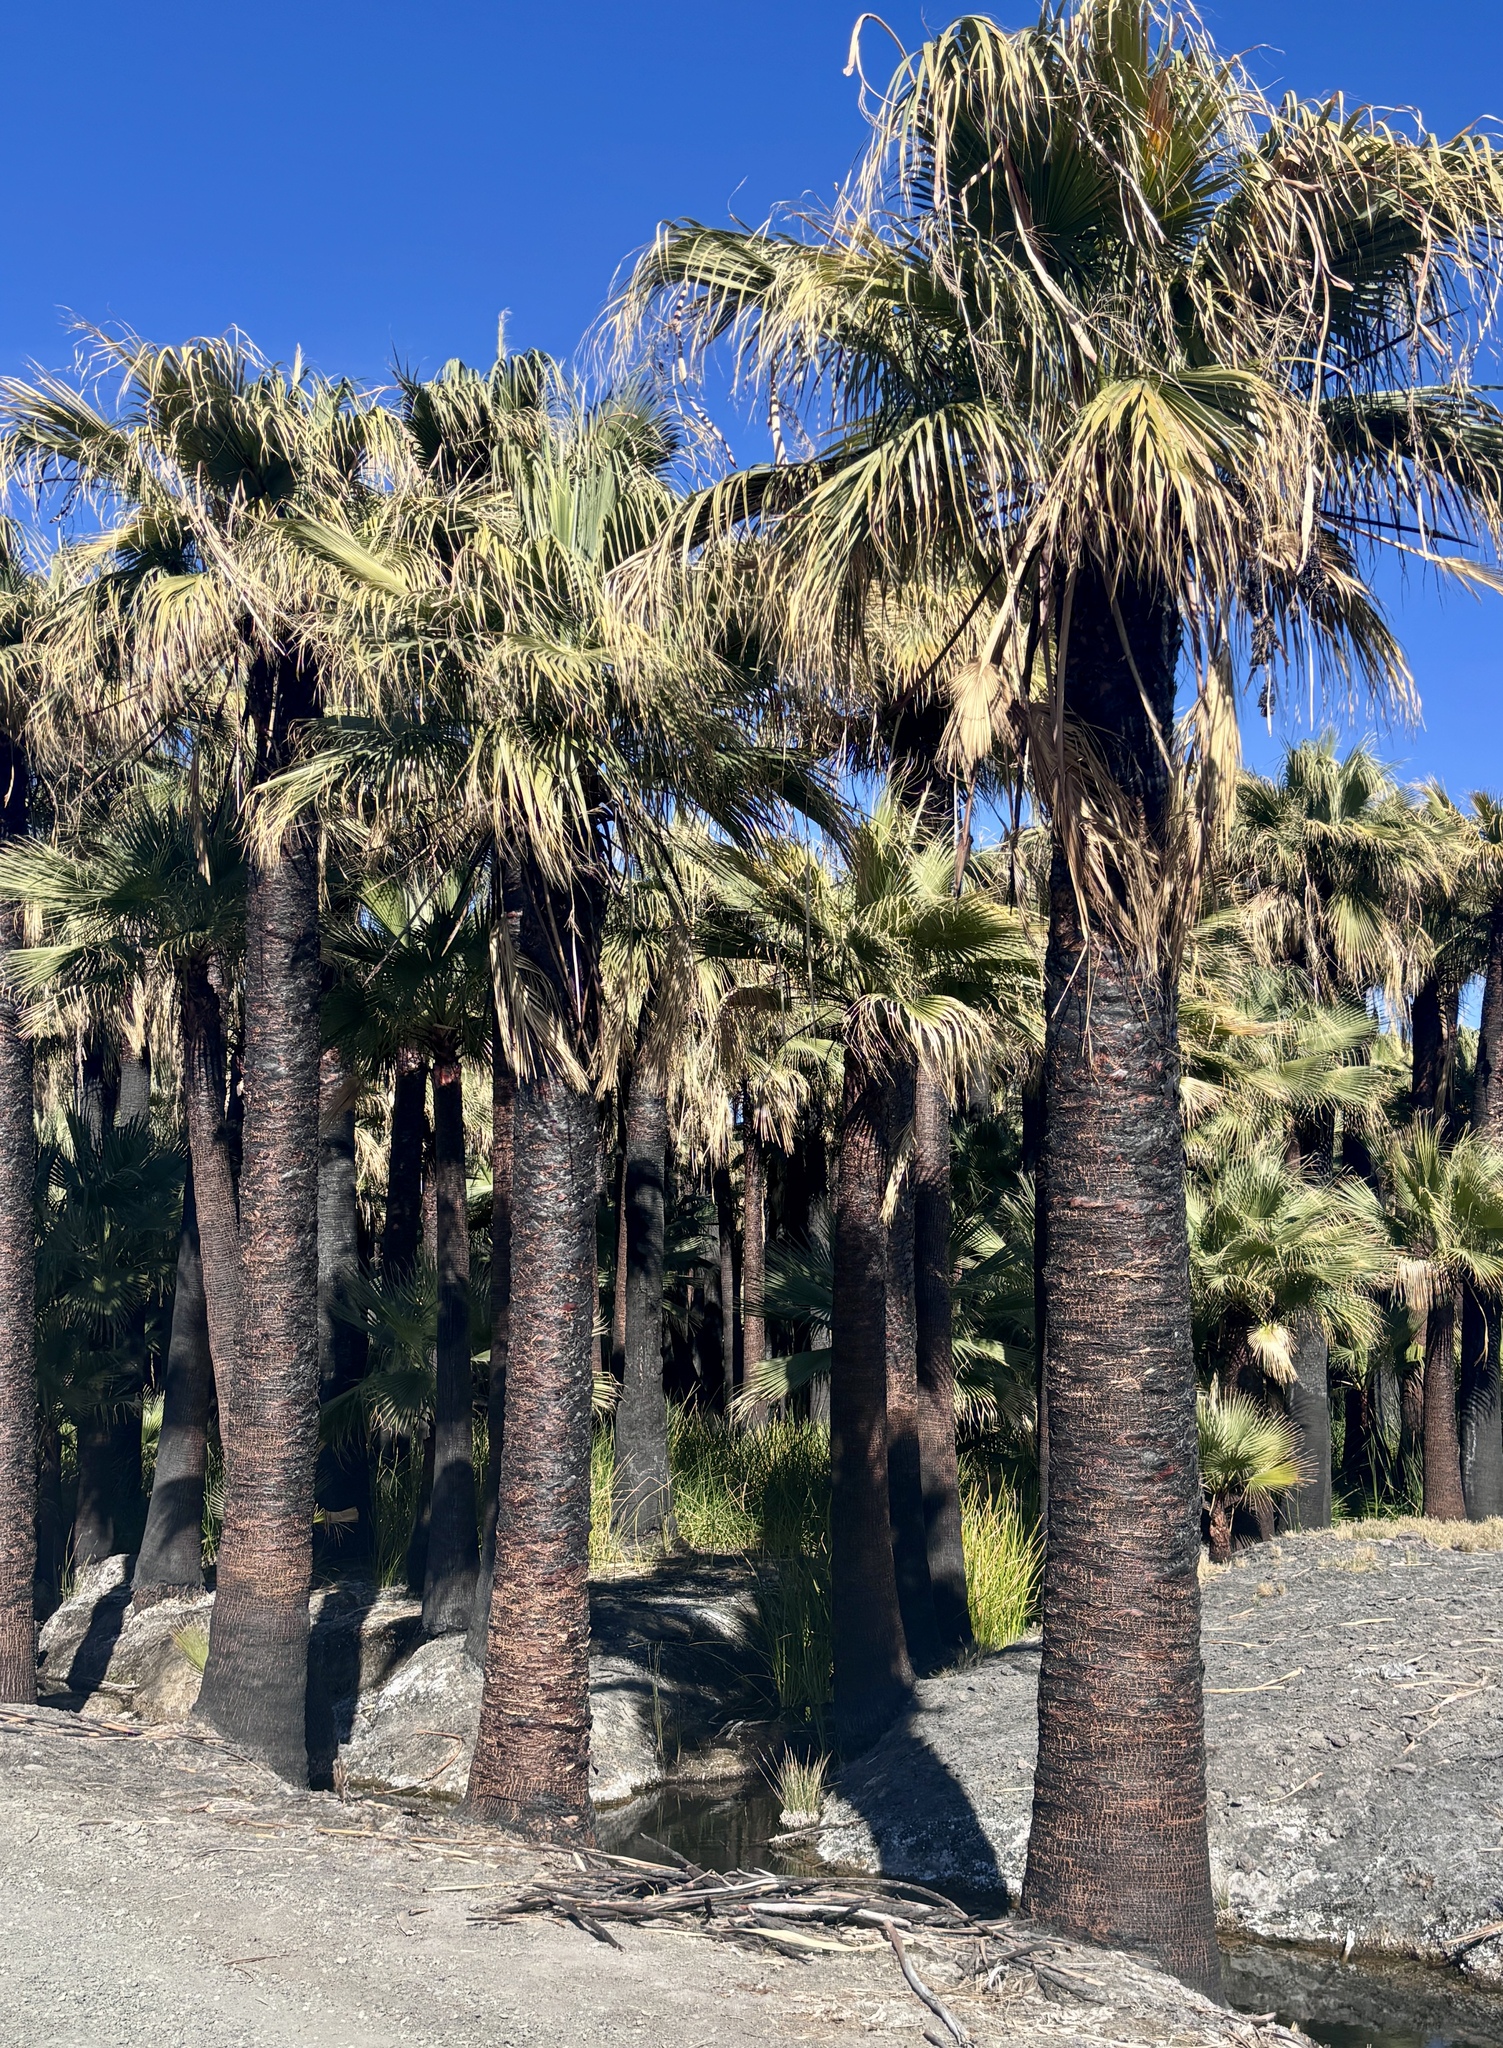
Flower and fruit production nearly doubles in crown-scorched trees during the first postfire growing season [8,32].

A stand of severely burned California palms less than a month after the February 2024 Palmas Fire, Riverside County, California. (CC BY-NC 4.0)

A stand of California palms 11 months after the February 2024 Palmas fire, Riverside County, California, showing vigorous regrowth of the crowns. (CC BY-NC 4.0)
Fire Regimes
Human-caused and natural fires are important factors affecting California palm and the oases in which they grow. A survey of oases along the San Andreas Fault revealed fire effects on palms at all sites. Prior to the nineteenth century, Native Americans practiced fire management in oases, burning them at intervals of about 4 years [40]. Burning increased the yield of fruit crops, removed the dead shag from trunks for easier access to crops, and removed understory phreatophytes competing for water resources. Spring flows increased, which temporarily reduced the high alkalinity of soils and favored California palm seed germination and seedling growth. The oases were thusly maintained at pioneer or early seral conditions [25,40].
Naturally-occurring oases fires are usually ignited by lightning strikes; natural average fire frequency is undocumented. Oases fire records show that fire can occur at any time of year. Oases fuels are usually so prodigious and desiccated that lightning readily produces fire even when occurring in winter during heavy rain [40]. Other possible causes of natural fire have been suggested, including ignition from sparks given off by falling rock in canyon sites, and spontaneous combustion. Hydric portions of oases support dense growth with heavy accumulations of litter [39]. Spontaneous combustion occurs naturally in Louisiana marshes [38], and hydric portions of oases are similar in composition and environment [40].
For additional fire regime information, search FEIS for this species by entering the species name on the Advanced Search page and selecting “Fire Regime” as the publication type.
Fire Management Considerations
Fire is an essential element of California palm regeneration and oasis maintenance. Fire suppression, practiced in many oases for over 60 years, has resulted in dense understories of brush and young palms. The Thousand Palms Oasis, for example, located in the Colorado Desert, California, developed very little understory for 10 to 15 years following its last fire. Saltgrass was the understory pioneer. It was displaced by a dense growth of mesquite (Prosopis glandulosa; P. pubescens) and goldenbush. After 35 years of fire suppression the oasis supported a dense, tall undergrowth with a humid microclimate. Litter accumulations were "massive" [40]. California palm's ability to resist fire under such highly flammable conditions is unknown. Managers are concerned that current fuel loading in many oases constitutes a severe fire hazard to palms, and that the next fire will kill substantial numbers of mature trees [1,40]. Manually removing portions of the understory, followed by natural prescribed and/or prescribed fire is recommended [1].
Fire kills desert palm borer beetle larvae near the trunk exterior [8].
Federal Status
No special status.
Other Status
No entry.
Importance to Wildlife and Livestock
Many animals live in close association with California palm. Amphibians such as the canyon tree frog and Pacific tree frog frequent the hydric zone and nearby boulders beneath palms. Various rodents use the palm's shag for cover. A species of rat snake (Elaphe rosalica) depends upon the shag for shelter and food (rodents). Oases attract numerous species of birds because of the relative abundance of food, shelter, and nesting sites as compared to open desert. Hooded orioles use fibers from older palm leaves as nesting material [32], often constructing nests within the palms [11]. Gray fox and various birds and rodents eat the fruit, and the fruit is the main component in the fall diet of coyote [6,32,40,].
California palm oases were used as cattle rangeland from 1911 to 1913, and were grazed by sheep in the late 1940's [40].
Palatability and Nutritional Value
California palm fruits, including seeds, contain 348 calories per 100 grams. Percentages by weight of several nutrients in fruits (including seeds) are as follows [8]:
| Nutrient | Percent |
|---|---|
| Protein | 3.1 |
| Fat | 2.8 |
| Carbohydrate | 77.7 |
| Fiber | 10.4 |
| Ash | 5.4 |
Milligrams per 100 grams of several other nutrients in fruits (including seeds) are as follows [8]:
| Nutrient | Milligrams/100g |
|---|---|
| Calcium | 110 |
| Phosphorus | 89 |
| Iron | 7.8 |
| Carotene | 180 |
| Thiamine | 0.06 |
| Vitamin C | 0.13 |
| Niacin | 1.0 |
| Riboflavin | 0.13 |
Cover Value
No entry.
Value for Rehabilitation or Restoration of Disturbed Sites
No entry.
Other Uses
California palm is greatly valued as a landscaping ornamental [12].
Kamia and Cahuilla Indians selected California palm oases for village sites. The oases provided sources of water, food, and shade. California palm vegetative buds, flowers, and fruits were utilized as food. The fruits, resembling commercial dates in taste, were eaten fresh or dried; some dried fruit was made into meal. Leaves were used as thatching. Sandals, clothing, and baskets were fashioned from leaf fibers. Spoons and hunting bows were made from the petioles. The wood was used for kindling. Because of historical use by Indians, California palm oases are important archeological sites [25,26,32].
Other Management Considerations
Many California palm oases have been destroyed by agricultural and urban development. Others have been eliminated due to loss of oases water sources. California palm is sensitive to any change in water level; either a lowering of water tables or the inundation of root systems may kill plants [40]. Groundwater pumping by the town of Twenty-nine Palms, California may be partially responsible for the 10-foot (3 m) drop in the water table at some sites of nearby Joshua Tree National Monument [1]. California palms in the Monument's Oasis of Mara are threatened by the drying up of the spring feeding the oasis [1,41]. Other phreatophytes competing for limited water resources can also greatly effect how much water will be available to palms. Increases of mesquite in the understory of the Oasis of Mara are probably an additional cause of the water table drop [1]. Saltcedar (Tamarix spp.), a strongly competitive exotic with an extremely high evapotranspiration rate, can dry up or reduce the yield of oases seeps and springs [4]. Saltcedar is displacing California palm in some areas [31,40]. See the FEIS write-up on Tamarix ramosissima for information regarding the control of saltcedar. Near the San Andreas Fault, palms receiving percolating water through rock fractures sometimes perish when the fault shifts, eliminating or relocating seeps [32].
Harmful agents: California palm is resistant to most fungal and bacterial infections [26]. A crown rot (Penicillium vermoeseni) sometimes infects trees that have been injured by lightning strikes or fire. Lightning-injured trees may be difficult to detect because palms do not generally show lightning disfigurement [18]. Palms, however, are occasionally decapitated by lightning [39]. California palm is the specific host of the giant palm borer beetle (Dynapate wrightii). Larvae of this insect feed on the wood [26,32] and can weaken or kill trees [8].
Outlying California palm oases are popular destinations for hikers, four-wheel drive, and dune-buggy enthusiasts. Vegetation disturbance, vandalism, and theft of Indian relics by unscrupulous recreationists are of continuing management concern [32].
Cultivation: California palm is easily grown from seed. The seed is abundant; it stores and germinates well, and seedlings transplant easily [12,25]. Information on seed processing, storage, and germination techniques and seedling care is available [19].
Table A1— Forest and range ecosystems, Bureau of Land Management (BLM) physiographic regions, Kuchler plant associations, Society for American Foresters (SAF) forest cover types, and Society for Rangeland Management (SRM) rangeland cover types in which this species occurs.
Forest and Range Ecosystems (Garrison et al. 1977)
- FRES30 Desert shrub
BLM Physiographic Regions (Bernard and Brown 1977)
- 7 Lower Basin and Range
Kuchler Plant Associations (Kuchler 1964)
- K027 Mesquite bosque
- K040 Saltbush - greasewood
- K041 Creosotebush
- K042 Creosotebush - bursage
- K043 Paloverde - cactus shrub
SAF Cover Types (Eyre 1980)
- 242 Mesquite
SRM Rangeland Cover Types (Shiflet 1994)
- No entry
1. Agee, James K. 1974. Fire management in the National Parks. Western Wildlands. 1(3): 27-33. [18558]
2. Bernard, Stephen R.; Brown, Kenneth F. 1977. Distribution of mammals, reptiles, and amphibians by BLM physiographic regions and A.W. Kuchler's associations for the eleven western states. Tech. Note 301. Denver, CO: U.S. Department of the Interior, Bureau of Land Management. 169 p. [434]
3. Bomhard, Miriam L. 1950. Palm trees in the United States. Information Bulletin No. 22. Washington, DC: U.S. Department of Agriculture. 26 p. [17162]
4. Gartner, F. Robert. 1977. Ecological changes on pine grassland burned in fall and spring. Final Report Contract No. PX 120051027, U.S. Department of the Interior National Park Service, Rocky Mountain Regional Office. Rapid City, SD: South Dakota State University, Agricultural Research and Extension Center. 35 p. [1001]
5. Horton, J. S.; Kraebel, C. J. 1955. Development of vegetation after fire in the chamise chaparral of southern California. Ecology. 36(2): 244-262. [3737]
6. Bullock, Stephen H. 1980. Dispersal of a desert palm by opportunistic frugivores. Principes. 24(1): 29-32. [19703]
7. Cornett, James W. 1983. The occurrence of the desert fan palm, Washington filifera, in southern Nevada. Desert Plants. 5(3): 169-172. [2985]
8. Cornett, James W. 1985. Germination of Washingtonia filifera seeds eaten by coyotes. Principes. 20(1): 19. [19220]
9. Cornett, James W. 1987. Cold tolerance in the desert fan palm, Washingtonia filifera (Arecaceae). Madrono. 34(1): 57-62. [19913]
10. Cornett, James W. 1987. Nutritional value of desert fan palm fruits. Principes. 31(4): 159-161. [19918]
11. DeGraaf, Richard M.; Scott, Virgil E.; Hamre, R. H.; [and others]. 1991. Forest and rangeland birds of the United States: Natural history and habitat use. Agric. Handb. 688. Washington, DC: U.S. Department of Agriculture, Forest Service. 625 p. [15856]
12. DeMason, Darleen A. 1988. Seedling development in Washingtonia filifera (Arecaceae). Botanical Gazette. 149(1): 45-56. [4476]
13. Eyre, F. H., ed. 1980. Forest cover types of the United States and Canada. Washington, DC: Society of American Foresters. 148 p. [905]
14. Garrison, George A.; Bjugstad, Ardell J.; Duncan, Don A.; [and others]. 1977. Vegetation and environmental features of forest and range ecosystems. Agric. Handb. 475. Washington, DC: U.S. Department of Agriculture, Forest Service. 68 p. [998]
15. Holland, Robert F. 1986. Preliminary descriptions of the terrestrial natural communities of California. Sacramento, CA: California Department of Fish and Game. 156 p. [12756]
16. Kearney, Thomas H.; Peebles, Robert H.; Howell, John Thomas; McClintock, Elizabeth. 1960. Arizona flora. 2d ed. Berkeley, CA: University of California Press. 1085 p. [6563]
17. Khan, M. I. 1982. Allelopathic potential of dry fruits of Washingtonia filifera (L. Linden) H. Wendl. II. Inhibition of seedling growth. Biologia Plantarum (Praha). 24(4): 275-281. [19886]
18. Komarek, E. V., Sr. 1965. Fire ecology-grasslands and man. In: Proceedings, 4th annual Tall Timbers fire ecology conference; 1965 March 18-19; Tallahassee, FL. Tallahassee, FL: Tall Timbers Research Station: 169-220. [18921]
19. Krugman, Stanley L. 1974. Washingtonia filifera (Linden) H.Wendl. California washingtonia. In: Schopmeyer, C. S., ed. Seeds of woody plants in the United States. Agriculture Handbook No. 450. Washington: U. S. Department of Agriculture, Forest Service: 855-856. [7778]
20. Kuchler, A. W. 1964. Manual to accompany the map of potential vegetation of the conterminous United States. Special Publication No. 36. New York: American Geographical Society. 77 p. [1384]
21. Lotan, James E.; Brown, James K. 1984. Fire's effects on wildlife habitat--symposium proceedings;. 1984 March 21; Missoula, MT. General Technical Report INT- 186. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station; 1985. 96 p. [1476]
22. McClenaghan, Leroy R., Jr.; Beauchamp, Arthur C. 1986. Low genic differentiation among isolated populations of the California fan palm (Washingtonia filifera). Evolution. 40(2): 315-322. [3260]
23. Mayeux, Herman S., Jr. 1987. Application of herbicides on rangelands with a carpeted roller: timing of treatment in dense stands of honey mesquite. Journal of Range Management. 40(4): 348-352. [29]
24. Munz, Philip A. 1974. A flora of southern California. Berkeley, CA: University of California Press. 1086 p. [4924]
25. Lohmiller, Robert George. 1963. Drought and its effect on condition and production of a desert grassland range. University Park, NM: New Mexico State University. 57 p. M.S. thesis. [2715]
26. Parish, S. B. 1907. A contribution toward a knowledge of the genus Washingtonia. Botanical Gazette. 44: 408-433. [3063]
27. Parish, S. B. 1930. Vegetation of the Mohave and Colorado Deserts of southern California. Ecology. 11(3): 481-499. [15095]
28. Preston, Richard J., Jr. 1948. North American trees. Ames, IA: The Iowa State College Press. 371 p. [1913]
29. Raunkiaer, C. 1934. The life forms of plants and statistical plant geography. Oxford: Clarendon Press. 632 p. [2843]
30. Roberts, Warren G.; Howe, J. Greg; Major, Jack. 1980. A survey of riparian forest flora and fauna in California. In: Sands, Anne, editor. Riparian forests in California: Their ecology and conservation: Symposium proceedings. Davis, CA: University of California, Division of Agricultural Sciences: 3-19. [5271]
31. Rodman, John. 1990. Reflections on tamarisk bashing. In: Hughes, H. Glenn; Bonnicksen, Thomas M., eds. Restoration '89: the new management challenge: Proceedings, 1st annual meeting of the Society for Ecological Restoration; 1989 January 16-20; Oakland, CA. Madison, WI: The University of Wisconsin Arboretum, Society for Ecological Restoration: 59-68. [14688]
32. Schwenkmeyer, Dick. 1986. The palm oasis: our tropical vestige. Environment Southwest. 514: 18-23. [5606]
33. Shantz, H. L.; Piemeisel, R. L. 1924. Indicator significance of the natural vegetation of the Southwestern desert region. Journal of Agricultural Research. 28(8): 721-803. [12222]
34. Szaro, Robert C. 1989. Riparian forest and scrubland community types of Arizona and New Mexico. Desert Plants. 9(3-4): 70-138. [604]
35. Thorne, Robert F. 1976. The vascular plant communities of California. In: Latting, June, ed. Symposium proceedings: plant communities of southern California; 1974 May 4; Fullerton, CA. Special Publication No. 2. Berkeley, CA: California Native Plant Society: 1-31. [3289]
36. Tomlinson, P. B. 1960. Essays on the morphology of palms. I. Germination and the seedling. Principes. 4: 56-61. [19917]
37. U.S. Department of Agriculture, Soil Conservation Service. 1982. National list of scientific plant names. Vol. 1. List of plant names. SCS-TP-159. Washington, DC. 416 p. [11573]
38. Viosca, Percy, Jr. 1931. Spontaneous combustion in the marshes of southern Louisiana. Ecology. 12(2): 439-443. [14582]
39. Vogl, Richard J. 1967. Fire adaptations of some southern California plants. In: Proceedings, Tall Timbers fire ecology conference; 1967 November 9-10; Hoberg, California. No. 7. Tallahassee, FL: Tall Timbers Research Station: 79-109. [6268]
40. Vogl, Richard J.; McHargue, Lawrence T. 1966. Vegetation of California fan palm oases on the San Andreas Fault. Ecology. 47(4): 532-540. [3044]
41. Holden, M. 1993, pers. comm.