


Ribes lacustre, prickly currant
Carey, Jennifer H. 1995. Ribes lacustre, prickly currant. In: Fire Effects Information System, [Online]. U.S. Department of Agriculture, Forest Service, Rocky Mountain Research Station, Fire Sciences Laboratory (Producer). Available: https://research.fs.usda.gov/feis/species-reviews/riblac
| Abbreviation | Common Name | Scientific Name | Classification | Status |
|---|---|---|---|---|
| Plants | ||||
| RIBLAC | prickly currant | Ribes lacustre | Life Form: Plants/Shrub Kingdom: Plantae Class: Dicot Order: Rosales Family: Grossulariaceae Genus: Ribes | Fed. Protected: No Nativity: Native Invasiveness: Noninvasive |


Taxonomy
The scientific name of prickly currant is Ribes lacustre (Pers.) Poir. (Grossulariaceae) [25,33,34,35,59]. There are no currently accepted infrataxa.
Synonyms
None
Other Common Names
bristly black currant, swamp currant
General Distribution

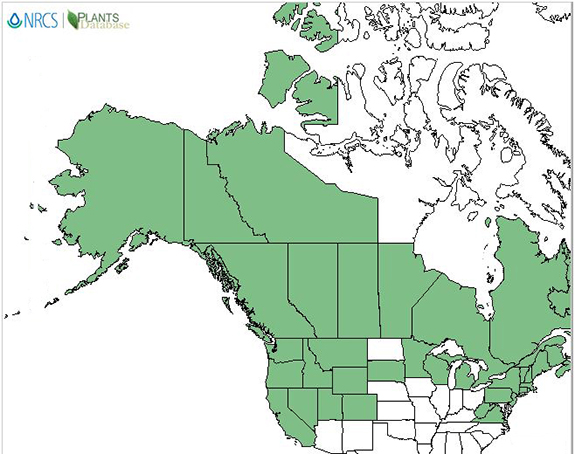
Distribution of prickly currant.
Prickly currant occurs throughout Canada from Newfoundland to Yukon Territory and in Alaska [35,54,59]. It extends south into the continental United States in the Coast and Cascade ranges to northern California, in the Rocky Mountains to central Colorado and northern Utah, in the Great Lake States, and in the Appalachian Mountains to West Virginia [8,25,33,65,72]. In the northern Great Plains region, prickly currant occurs in the Black Hills [26].
States and Provinces
- United States: AK, CA, CO, CT, ID, ME, MA, MI, MN, MT,NH, OH, OR, PA, SD, UT, VT, VA, WA, WV, WY
- Canada: AB, BC, MB, NB, NF, NT, ON, PE, PQ, SK, YT
Site Characteristics
Prickly currant occurs in moist woods and forests, ravines, shrub thickets, meadow margins, swamps, rock crevices, seepage areas, along avalanche chutes, on streambanks, and on steep slopes [4,27,33,34,59]. On Big Snowy Peak in central Montana, prickly currant grows in crevices of limestone outcrops and cliffs [5].
Prickly currant occurs in cool, moist climates. It occurs from 7,700 to 10,500 feet (2,300-3,200 m) in Utah, 7,000 to 11,400 feet (2,100-3,500 m) in Colorado, 5,500 to 10,700 feet (1,700-3,300 m) in Wyoming, and 3,000 to 8,700 feet (900-2,700 m) in Montana [17]. At the southern extremes of its range (California, Utah, Colorado, and West Virginia), prickly currant occurs in cool high-elevation forests [1,56,65]. It is found more often on northerly and easterly exposures than southerly or westerly exposures [44].
Prickly currant occurs on moist, nutrient-rich sites. In 91- to 160-year-old lodgepole pine (Pinus contorta) stands and 60- to 160-year-old white spruce (Picea glauca) stands in west-central Alberta, prickly currant had significantly (P<0.025) higher canopy cover on sites with high site index (indicative of higher productivity) than low site index [66]. In the Prince Rupert Forest Region of British Columbia, prickly currant occurs on mesic to subhydric sites with high nutrient status (permesotrophic to subeutrophic) [73]. It occurs in both acidic and basic soils [1,5].
Plant Communities
Prickly currant occurs in woods, forests, and shrublands. It is a common but not abundant understory species [16,27,32].
Prickly currant occurs in the understory of subalpine forests in Wyoming with gooseberry currant (Ribes montigenum), sidebells wintergreen (Orthilia secunda), heartleaf arnica (Arnica cordifolia), and fireweed (Epilobium angustifolium) [9].
In the cedar (Thuja spp.)-hemlock (Tsuga spp.) zone of northwestern British Columbia, prickly currant occurs with devil's club (Oplopanax horridus), leafy moss (Mnium spp.), oak fern (Gymnocarpium dryopteris), Schreber's moss (Pleurozium schreberi), common ladyfern (Athyrium filix-femina), and horsetail (Equisetum spp.) [28]. Prickly currant occurs in the oak fern, devil's club, horsetail, and queencup beadlily (Clintonia uniflora) series of the wet, cool subboreal spruce (Picea spp.) forest zone in British Columbia [32].
Prickly currant occurs with Rocky Mountain maple (Acer glabrum), Utah honeysuckle (Lonicera utahensis), blue huckleberry (Vaccinium membranaceum), and western meadowrue (Thalictrum occidentale) in the understory of a virgin grand fir (Abies grandis) forest in northern Idaho [36].
In spruce forests in Alberta, prickly currant occurs with other mesophytic species including twinberry honeysuckle (Lonicera involucrata), highbush cranberry (Viburnum edule), tall bluebells (Mertensia paniculata), wild sarsaparilla (Aralia nudicaulis), bluejoint reedgrass (Calamagrostis canadensis), oak fern, stiff clubmoss (Lycopodium amnotinum), and claspleaf twistedstalk (Streptopus amplexifolius) [41].
Prickly currant occurs in riparian woodlands and shrublands. It occurs in a thinleaf alder (Alnus incana ssp. tenuifolia) riparian dominance type in east-central Oregon [50].In the Klamath Mountains of northern California, prickly currant borders streams with thinleaf alder, California mountain-ash (Sorbus californica), and Scouler willow (Salix scouleriana), and it occurs in thickets with thinleaf alder, Sitka alder (Alnus viridis ssp. sinuata), red-osier dogwood (Cornus sericea), red elderberry (Sambucus racemosa ssp. pubens), and cascara (Rhamnus purshiana) [56].
Clearcuts in the Olympic Mountains in Washington, dominated by oceanspray (Holodiscus discolor) and thimbleberry (Rubus parviflorus), include common snowberry (Symphoricarpos albus) and prickly currant [23].
Botanical Description

Prickly currant flowers, Olympic National Park, Washington. (CC BY-NC 4.0)
Prickly currant is a native, deciduous shrub that grows 3 to 4 feet (1-1.2 m) tall [44,59,72]. In sunlight prickly currant grows erect, but in shade, branches are often reclining or trailing [44]. Prickly currant has prickly stems and nodal spines. The drooping raceme has 5 to 15 flowers [33]. The berries average 0.34 inch (8.6 mm) in diameter and contain an average of 16.5 small seeds [52].
The root systems of Ribes spp. consist of shallow roots radiating from a central root crown [47]. Prickly currant roots are very shallow, especially on moist sites, but lateral spread can be extensive [48]. Some sources report that prickly currant is rhizomatous [22,48] while others report that it is nonrhizomatous [61].Prickly currant partially buried by volcanic ejecta from Mount St. Helens in southern Washington had not developed rhizomes but had a well-developed adventitious root system [3].
Raunkiaer Life Form (Raunkiaer 1934)
- Phanerophyte
Seasonal Development
Prickly currant flowers from May to June, and berries ripen in August. Seeds germinate in the spring [51]. Prickly currant does not always produce fruit in spruce-fir (Abies spp.) forests of Canada because of the short growing season [27].
Regeneration Processes
Prickly currant regenerates primarily from seed. Plants first begin producing seeds when 3 to 5 years old. An average bush produces 50 to 75 berries. Good crops occur in 2- to 3-year intervals. Some seeds are dispersed by animals, but many berries fall to the ground beneath the parent plant [44].
Stratification is usually required to break the dormancy in prickly currant seed. Seeds stored at 32 degrees Fahrenheit (0 deg C) for 120 to 200 days had 48 percent germination in sand moistened with nutrient solution. Alternating diurnal temperatures (77 degrees Fahrenheit (25 deg C) and 41 or 50 degrees Fahrenheit [5 or 10 deg C]) results in some germination without prior stratification. Scarification enhances germination. A five-minute soak in 2 to 10 percent sulfuric acid solution improved germination [51].
Mineral soil is the best seed bed. Prickly currant establishes on well scarified sites [44,61].
Prickly currant seeds have long-term viability. They accumulate in the organic mantle and mineral soil over time. The mineral soil seedbank in mature forests in west-central Idaho contained 51 viable prickly currant and sticky currant (Ribes viscosissimum) seeds per square foot (567/sq m). Over 80 percent of the viable seeds were found in the top 2 inches (5 cm) of mineral soil. The two Ribes spp. were combined in the data because seedlings could not be distinguished in the greenhouse [39].
Prickly currant regenerates vegetatively [44,48]. Prickly currant stems in contact with soil produce adventitious roots [3,27,48]. In southern Washington, prickly currant that was partially buried for 1 year by 2 to 8 inches (5-20 cm) of volcanic ejecta had two to five adventitious roots per centimeter of stem. Maximum adventitious root length was 10 inches (25 cm) [3]. Offord and others [48] observed rhizomes in prickly currant near Mount Hood in northwestern Oregon. Some sources [22,43,47] suggest that prickly currant sprouts from the root crown, but definitive documentation was not found in the literature.
Successional Status
Prickly currant is moderately shade tolerant [32,44] but grows most vigorously in canopy openings [27]. It establishes in partial shade or full sun after disturbance and then persists in the understory of closed canopy forests and woods [10,44,61]. Seedlings are suppressed on sites with more than 75 percent of full shade [44]. Prickly currant established on a 1-year-old mudflow surface formed by the volcanic eruption of Mount St. Helens. The mudflow was reworked nonorganic substrate with no shallowly buried soil [30]
Dense thickets of prickly currant are uncommon. Prickly currant canopy cover reported in the literature is generally less than 10 percent and commonly less than 1 percent [16,27,32].
Prickly currant response to timber harvest is an indicator of its successional status. Although prickly currant generally increases after clearcutting [2,20,23,32], its response is varied. In western Montana prickly currant cover averaged 1.5 percent in 7- to 16-year-old clearcuts but was only a trace in uncut stands [2]. In northern British Columbia, prickly currant increased in abundance on alluvial and poorly drained sites following clearcutting [20]. Prickly currant is a principal understory species on clearcuts in northwestern Washington [23]. In subalpine forests in central Colorado, pre- and postlogging prickly currant canopy cover was not significantly (P<0.05) different [13]. In northwestern Montana, prickly currant response to clearcutting depended on habitat type. In the subalpine fir/queencup beadlily habitat type, prickly currant canopy cover was lower on burn sites, clearcut sites, and avalanche chutes than on old growth sites; in the more mesic subalpine fir/menziesia (Menziesia spp.) habitat type, prickly currant canopy cover was higher after these disturbances than on old-growth sites [74].
Immediate Fire Effects
Fire that burns the organic soil probably kills prickly currant. Noste and Bushey [47] report that fire that removes the organic soil layer will likely kill the shallow root systems of most Ribes spp. Prickly currant was nearly absent from study sites after a severe prescribed fire in central Idaho (see Fire Case Studies) [42]. Low-severity fire probably top-kills prickly currant.
Prickly currant seeds contained in the organic mantle are destroyed by severe fire [44]. However, seeds buried in mineral soil probably survive most fire.
Postfire Regeneration Strategy (Stickney 1989)
- Ground residual colonizer (on-site, initial community)
- Secondary colonizer - off-site seed
Fire Adaptations
Prickly currant occurs in many forest types, such as grand fir and Engelmann spruce (Picea engelmannii)-subalpine fir (Abies lasiocarpa), that are characterized by long fire-free intervals punctuated by severe, stand-replacing fires [22,77]. The ability of prickly currant to regenerate after fire from long-lived seed stored in soil or from off-site sources makes prickly currant fairly resilient to stand-replacing fire [89]. Low-severity fire is probably more favorable to Ribes spp. than severe fire [78].
After fire prickly currant canopy cover increases slowly, reaching a maximum density in several to many decades [15,42,76]. Prickly currant cover was reported for sites with a history of fire in the southern boreal forest region of Quebec. Postfire ages of sites ranged from 26 to 230 years. Prickly currant was present on all sites at low cover. The highest prickly currant cover recorded (2.2 percent) occurred on the site with a postfire age of 74 [15]. The percent prickly currant cover follows:
| Year since fire | 26 | 46 | 74 | 120 | 143 | 167 | 174 | 230 |
| Canopy cover | 0.1 | 0.2 | 2.2 | 1.0 | 0.3 | 0.1 | 0.1 | 0.1 |
Plant Response to Fire
Numerous secondary sources suggest that prickly currant sprouts from the root crown and rhizomes after top-kill by fire [7,12,22,43, 47,77]. However, primary documentation of prickly currant sprouting from the root crown or rhizomes after fire was not found in the literature.
Prickly currant was present in the postfire ravine vegetation 1 year after a mid-summer wildfire in western Montana. Although the fire was generally severe, some ravine sites did not burn severely because of the higher moisture content of plant material and soil. Prickly currant plants recovered quickly in low-severity burn patches; the mechanism of recovery (sprouting from rootstocks, rhizomes, or adventitious stem buds) was not reported. Maximum prickly currant postfire canopy cover was 2.5 percent 1 year after fire and 6.3 percent 2 years after fire [37].
Prickly currant colonizes burned sites via long-lived buried seed and/or seed carried on to the site by animals [64]. Regeneration success after fire depends on site conditions and fire severity. Severe fire substantially reduces or delays prickly currant establishment [42]. Prickly currant seedlings were present on 1 of 18 burn sites 1 year after the Sundance wildfire in northern Idaho. The fire consumed the overstory, litter and duff; fire intensity ranged from 3,400 to 22,500 British thermal units per second per foot [63]. According to Steele and Geier-Hayes [61], prickly currant and sticky currant are common on scarified portions of past pile-and-burn sites but rare on severely burned areas. In western Montana black currant was 25.6 percent less frequent on burned slash pile sites than on adjacent unburned scarified clearcut sites. Postfire age of sampled burned sites averaged 8.8 years [70].
Optimal conditions for prickly currant establishment may not occur until several years after fire. In broadcast-burned clearcuts in north-central Idaho, prickly currant occurred in only 1 of 10 microplots in 1-year-old burns but was found on seven of nine microplots in 3-year-old burns [75]. Severe hot or dry soil conditions associated with some burns may discourage immediate colonization by prickly currant. Lyon [42] suggests that optimal environmental conditions for prickly currant establishment may not occur on some sites until other vegetation is established.
Prickly currant recovery was slow after prescribed broadcast fires in clearcut western larch (Larix occidentalis)-Douglas-fir (Pseudotsuga menziesii) forests in northwestern Montana. Prickly currant disappeared from the most severely burned site (E-8), but appeared within 8 years on three sites on which it had not been present in the prefire vegetation. Prickly currant pre- and postfire canopy cover follows [62]:
| Site | Prefire cover (%) | Year since fire | Postfire duff (cm) | |||||||
|---|---|---|---|---|---|---|---|---|---|---|
| 1 | 2 | 3 | 4 | 5 | 6 | 7 | 8 | |||
| N-6 | — | — | — | 1 | 1 | 1 | — | — | — | 7.0 |
| N-8 | — | — | — | — | — | 1 | — | 1 | 3 | 6.0 |
| E-8 | 1 | — | — | — | — | — | — | — | — | 6.6 |
| S-2 | 1 | — | — | — | — | — | 1 | — | — | Not reported |
| W-3 | — | — | — | — | — | — | — | — | 1 | 4.5 |
Literature that contains fire response information for Ribes spp. in general should be viewed with caution because of substantial differences between co-occurring species. In the above-mentioned study [62], sticky currant rapidly colonized some burned sites, reaching a maximum canopy cover of 11 percent after 4 years on a site from which it was absent before fire [62]. Lyon [42] also documented rapid sticky currant recovery after fire (see Fire Case Studies). Mueggler [45] combined Ribes spp. when he reported they were considerably more frequent on burn sites than unburned sites in grand fir and western redcedar (Thuja plicata) forest associations in northern Idaho. Prickly currant and sticky currant co-occur in these forests [14], and it is possible that only sticky currant was doing well on burned sites in the first several postfire years.
In north-central Idaho, the vegetation was measured for 36 clearcut and broadcast burned sites and 7 old-growth sites. Postfire ages of burned sites ranged from 1 to 23 years. Prickly currant average percent canopy volume (percent of total volume occupied in a 1x1x3 m space) and average height by postfire year follow [75]:
| Measured growth | Years since fire | Old Growth | ||||
|---|---|---|---|---|---|---|
| 1 | 3 | 8 | 12 | 23 | ||
| Avg. % canopy volume | 0.1 | 0.1 | 0.3 | 0.8 | — | trace |
| Average height (cm) | 11 | 24 | 45 | 65 | 43 | 25 |
Fire Regimes
For fire regime information, search FEIS for this species by entering the species name on the Advanced Search page and selecting “Fire Regime” as the publication type.
Fire Management Considerations
Nutrient content of shrub species was estimated for seven silvicultural treatments including burning in the Coram Experimental Forest in northwestern Montana [60]. The elemental content of prickly currant branches and leaves collected in July and August is presented [60].
Sawtooth National Forest, Idaho, prescribed fire study: Effects on prickly currant
Source
Lyon, L. Jack. 1971. Vegetal development following prescribed burning of Douglas-fir in south-central Idaho. Res. Pap. INT-105. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 30 p. [42].
Season/Severity Classification
Summer/severe
Study Location
The study site is located in Neal Canyon, 6 miles (9.6 km) north of Ketchum, Idaho, in the Sawtooth National Forest.
Prefire Vegetative Community
The study site was selectively logged in 1950 and 1960. The remaining trees were primarily pole and sapling Douglas-fir (Pseudotsuga menziesii), many of which were diseased. Minor tree species included lodgepole pine (Pinus contorta), subalpine fir (Abies lasiocarpa), Engelmann spruce (Picea engelmannii), and quaking aspen (Populus tremuloides). Understory vegetation was dominated by Rocky Mountain maple (Acer glabrum) and mountain snowberry (Symphoricarpos oreophilus). Prickly currant was a minor species.
Vegetation layers over and under 18 inches (46 cm) in height were sampled and described separately. Prickly currant under 18 inches occurred on 20 percent of the study quadrats. Prickly currant abundance of plants over 18 inches in height was:
| Density | 0.9 plant/1,000 ft² |
| Canopy cover | 0.67 % |
| Aerial crown volume | 16.8 ft³/1,000 ft² |
Target Species Phenological State
Prickly currant was probably in flowering and fruiting stages on August 1, the day of the fire.
Site Description
The mountainous study site is at 6,500 feet (1,980 m) elevation. Annual precipitation is from 14 to 17 inches (360-430 mm), most occurring in the winter as snow. The slope averages 64 percent and the aspect is 10 to 20 degrees. The soils are rocky, averaging 50 percent gravel.
Fire Description
The fire was started at 8 a.m. on August 1, 1963 and burned until 5 p.m. Air temperature was 50 degrees Fahrenheit (10 deg C) in the morning and nearly 80 degrees Fahrenheit (27 deg C) in the afternoon. Relative humidity declined from 50 percent in the morning to 10 percent in the afternoon. Fuel moisture sticks indicated 5 to 6 percent moisture. Surface winds were less than 5 miles per hour, but fire-induced gusts up to 30 miles per hour were recorded.
The fire was severe and crowned. All litter, herbaceous plants, dead woody stems less than 3 inches (7.6 cm) in diameter, and live woody stems less than 2 inches (5.1) in diameter were consumed. The Douglas-fir overstory was killed. The mean heat flux, measured using water-can integrating devices, was 200 calories per second for 45 seconds.
Fire Effects on Target Species
Prickly currant was killed by the fire. Prickly currant was observed on the study site beginning in postfire year 2. However, no prickly currant less than 18 inches in height was detected during the 7 postfire years in 2- by 2-foot quadrats. Density, height, and crown volume for prickly currant over 18 inches in height was originally recorded using quarter-point sampling [79], but this technique was eventually deemed inadequate because of low plant densities. Beginning in 1966 (postfire year 3), 0.04 acre (0.016 ha) plots were sampled, both in the original quarter-point sampling area and in three additional subplots located at lower, middle, and upper slope sites; measurable quantities of prickly currant occurred only on the lower and upper slope subplots. Prickly currant over 18 inches in height was first recorded in postfire year 3, presumably growing from seed in the first or second postfire year. The following data should be interpreted with caution because of very low sample numbers for prickly currant.
| Postfire year | Plants/1,000 ft² | Canopy cover (%) | Aerial crown volume (ft³/1,000 ft²) | ||||
|---|---|---|---|---|---|---|---|
| Original study area: | Subplots (lower slopes) | Subplots (upper slopes) | Original study area | Original study area | Subplots (lower slopes) | Subplots (upper slopes) | |
| 1 | — | * | * | — | — | * | * |
| 2 | — | * | * | — | — | * | * |
| 3 | T | 0.2 | 0.1 | T | 0.1 | 0.2 | 0.7 |
| 4 | T | 0.2 | 0.5 | 0.01 | 0.1 | 0.4 | 2.0 |
| 5 | — | 1.0 | 0.2 | — | 0.01 | 2.6 | 1.4 |
| 6 | 0.3 | 1.3 | 0.2 | 0.05 | 1.1 | 7.4 | 1.8 |
| 7 | 0.1 | 1.8 | 0.5 | T | T | 4.4 | 2.5 |
| *Data were not collected | |||||||
Height and crown volume were measured and averaged for the first four prickly currants on the burn to reach 18 inches in height.
| Measured Growth | Postfire year | ||||||
|---|---|---|---|---|---|---|---|
| 1 | 2 | 3 | 4 | 5 | 6 | 7 | |
| Average height (ft) | — | — | 1.7 | 1.6 | 1.5 | 2.4 | 1.9 |
| Average volume (ft³) | — | — | 2.6 | 3.1 | 4.4 | 11.5 | 6.2 |
A wildfire site which burned in 1950 was located near the Neal Canyon study site. Twenty years after the wildfire, prickly currant averaged 2.6 plants per 1,000 square feet, 0.6 percent cover , and 12.2 cubic feet aerial crown volume per 1,000 square feet. Based on the Neal Canyon prescribed fire and the wildfire, Lyon [42] projects that prickly currant will reach prefire crown volumes 30 to 40 years after fire.
Fire Management Implications
No entry.
Federal Status
None
Other Status
No entry.
Importance to Wildlife and Livestock
Prickly currant berries are eaten by rodents, bears, and birds [38]. In southwestern Alberta grizzly bears feed on prickly currant berries in late summer and early autumn [31]. Elk, mule deer, white-tailed deer, and mountain goats eat prickly currant foliage [11,18,55,58,71]. In Montana prickly currant was 1 percent of elk diet in early summer and 3 percent in late summer [18].
Palatability and Nutritional Value
Prickly currant browse is moderately palatable to livestock, elk, and deer [17,38]. The berries are edible but somewhat disagreeable tasting [35,38,59].
Prickly currant berries collected in the summer in northern Ontario consisted of 79.68 percent moisture, 20 percent dry matter, 0.28 percent fat, 1.46 percent protein, and 5.66 percent soluble carbohydrate based on fresh fruit weight. Fresh prickly currant fruit contains slightly more than 30 kilocalories per 100 grams [69].
Nutritional values of prickly currant berries collected in late summer in southeastern Washington, based on dry weight, were 2.94 percent protein, 4.09 percent lipid, 3.96 percent neutral detergent fiber, 4.56 percent ash, 0.282 percent calcium, 0.066 percent magnesium, 0.17 percent phosphorus, and 1.887 percent potassium [52].
Norton and others [46] analyzed the nutritional value of dried prickly currant berries stored for 1 year. Traditional Native American drying and storing methods were used. One gram dry weight contained on average 3.19 milligrams calcium, 0.05 milligram iron, 0.94 milligram magnesium, 0.02 milligram zinc, and 3.33 milligrams ascorbic acid [46].
Cover Value
In Wyoming, prickly currant is considered poor cover for elk and pronghorn and fair cover for mule deer and white-tailed deer. It is good cover for upland game birds, small nongame birds, and small mammals [17].
Value for Rehabilitation or Restoration of Disturbed Sites
No entry.
Other Uses
Native Americans in the Pacific Northwest eat prickly currant berries [46].
Other Management Considerations
Prickly currant is an alternate host for white pine blister rust (Cronartium ribicola) which infests five-needled pines. Because of its association with the rust, prickly currant has been a target of various eradication studies. Prickly currant is highly resistant to chemical injury [48]. Efforts to eradicate Ribes spp. have been unsuccessful and have not resulted in decreased rust infection. Only a few Ribes bushes per acre are sufficient to perpetuate blister rust [29].
Although prickly currant establishes on scarified ground after tree harvest, it does not impede conifer seedling establishment [61].
Grazing by wild ungulates prevents development of prickly currant in clearcuts. Eleven years after clearcutting, burned and unburned grazed sites averaged 0.3 percent cover prickly currant. Ungrazed burned clearcuts averaged 4.6 percent cover and ungrazed unburned clearcuts averaged 9.8 percent cover [19].
Table A1— Forest and range ecosystems, Bureau of Land Management (BLM) physiographic regions, Kuchler plant associations, Society for American Foresters (SAF) forest cover types, and Society for Rangeland Management (SRM) rangeland cover types in which this species occurs.
Forest and Range Ecosystems (Garrison et al. 1977)
- FRES11 Spruce-fir
- FRES18 Maple-beech-birch
- FRES19 Aspen-birch
- FRES20 Douglas-fir
- FRES22 Western white pine
- FRES23 Fir-spruce
- FRES24 Hemlock-Sitka spruce
- FRES25 Larch
- FRES26 Lodgepole pine
- FRES28 Western hardwoods
BLM Physiographic Regions (Bernard and Brown 1977)
- 1 Northern Pacific Border
- 2 Cascade Mountains
- 5 Columbia Plateau
- 8 Northern Rocky Mountains
- 9 Middle Rocky Mountains
- 10 Wyoming Basin
- 11 Southern Rocky Mountains
- 15 Black Hills Uplift
- 16 Upper Missouri Basin and Broken Lands
Kuchler Plant Associations (Kuchler 1964)
- K001 Spruce-cedar-hemlock forest
- K003 Silver fir-Douglas-fir forest
- K004 Fir-hemlock forest
- K007 Red fir forest
- K008 Lodgepole pine-subalpine forest
- K012 Douglas-fir forest
- K013 Cedar-hemlock-pine forest
- K014 Grand fir-Douglas-fir forest
- K015 Western spruce-fir forest
- K025 Alder-ash forest
- K093 Great Lakes spruce-fir forest
- K096 Northeastern spruce-fir forest
- K106 Northern hardwoods
SAF Cover Types (Eyre 1980)
- 60 Beech-sugar maple
- 107 White spruce
- 201 White spruce
- 205 Mountain hemlock
- 206 Engelmann spruce-subalpine fir
- 207 Red fir
- 208 Whitebark pine
- 210 Interior Douglas-fir
- 211 White fir
- 212 Western larch
- 213 Grand fir
- 215 Western white pine
- 218 Lodgepole pine
- 221 Red alder
- 222 Black cottonwood-willow
- 223 Sitka spruce
- 227 Western redcedar-western hemlock
SRM Rangeland Cover Types (Shiflet 1994)
- 422 Riparian
1. Allen, Robert B.; Peet, Robert K.; Baker, William L. 1991. Gradient analysis of latitudinal variation in Southern Rocky Mountain forests. Journal of Biogeography. 18(2): 123-138. [14875]
2. Antos, Joseph A.; Shearer, Raymond C. 1980. Vegetation development on disturbed grand fir sites, Swan Valley, northwestern Montana. Res. Pap. INT-251. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 26 p. [7269]
3. Antos, Joseph A.; Zobel, Donald B. 1985. Plant form, developmental plasticity and survival following burial by volcanic tephra. Canadian Journal of Botany. 63: 2083-2090. [12553]
4. Antos, Joseph A.; Zobel, Donald B. 1986. Habitat relationships of Chamaecyparis nootkatensis in southern Washington, Oregon, and California. Canadian Journal of Botany. 64: 1898-1909. [19168]
5. Bamberg, Samuel A.; Major, Jack. 1968. Ecology of the vegetation and soils associated with calcareous parent materials in three alpine regions of Montana. Ecological Monographs. 38(2): 127-167. [12554]
6. Bernard, Stephen R.; Brown, Kenneth F. 1977. Distribution of mammals, reptiles, and amphibians by BLM physiographic regions and A.W. Kuchler's associations for the eleven western states. Tech. Note 301. Denver, CO: U.S. Department of the Interior, Bureau of Land Management. 169 p. [434]
7. Bradley, Anne F.; Noste, Nonan V.; Fischer, William C. 1992. Fire ecology of forests and woodlands of Utah. Gen. Tech. Rep. INT-287. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 128 p. [18212]
8. Braun, E. Lucy. 1961. The woody plants of Ohio. Columbus, OH: Ohio State University Press. 362 p. [12914]
9. Clary, Warren P. 1983. Overstory-understory relationships: spruce-fir forests. In: Bartlett, E. T.; Betters, David R., eds. Overstory-understory relationships in Western forests. Western Regional Research Publication No. 1. Fort Collins, CO: Colorado State University Experiment Station: 9-12. [3310]
10. Cormack, R. G. H. 1953. A survey of coniferous forest succession in the eastern Rockies. Forestry Chronicle. 29: 218-232. [16458]
11. Cowan, Ian McTaggart. 1945. The ecological relationships of the food of the Columbian black-tailed deer, Odocoileus hemionus columbianus (Richardson), in the c. forest region southern Vancouver Island, British Columbia. Ecological Monographs. 15(2): 110-139. [16006]
12. Crane, M. F.; Fischer, William C. 1986. Fire ecology of the forest habitat types of central Idaho. Gen. Tech. Rep. INT-218. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 85 p. [5297]
13. Crouch, Glenn L. 1985. Effects of clearcutting a subalpine forest in central Colorado on wildlife habitat. Res. Pap. RM-258. Fort Collins, CO: U.S. Department of Agriculture, Forest Service, Rocky Mountain Forest and Range Experiment Station. 12 p. [8225]
14. Daubenmire, Rexford F.; Daubenmire, Jean B. 1968. Forest vegetation of eastern Washington and northern Idaho. Technical Bulletin 60. Pullman, WA: Washington State University, Agricultural Experiment Station. 104 p. [749]
15. De Grandpre, Louis; Gagnon, Daniel; Bergeron, Yves. 1993. Changes in the understory of Canadian southern boreal forest after fire. Journal of Vegetation Science. 4: 803-810. [23019]
16. Despain, Don G. 1973. Vegetation of the Big Horn Mountains, Wyoming, in relation to substrate and climate. Ecological Monographs. 43(3): 329-355. [789]
17. Dittberner, Phillip L.; Olson, Michael R. 1983. The plant information network (PIN) data base: Colorado, Montana, North Dakota, Utah, and Wyoming. FWS/OBS-83/86. Washington, DC: U.S. Department of the Interior, Fish and Wildlife Service. 786 p. [806]
18. Edge, W. Daniel; Marcum, C. Les; Olson-Edge, Sally L. 1988. Summer forage and feeding site selection by elk. Journal of Wildlife Management. 52(4): 573-577. [6778]
19. Edgerton, Paul J. 1987. Influence of ungulates on the development of the shrub understory of an upper slope mixed conifer forest. In: Provenza, Frederick D.; Flinders, Jerran T.; McArthur, E. Durant, compilers. Proceedings--symposium on plant-herbivore interactions; 1985 August 7-9; Snowbird, UT. Gen. Tech. Rep. INT-222. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station: 162-167. [7411]
20. Eis, S. 1981. Effect of vegetative competition on regeneration of white spruce. Canadian Journal of Forest Research. 11: 1-8. [10104]
21. Eyre, F. H., ed. 1980. Forest cover types of the United States and Canada. Washington, DC: Society of American Foresters. 148 p. [905]
22. Fischer, William C.; Clayton, Bruce D. 1983. Fire ecology of Montana forest habitat types east of the Continental Divide. Gen. Tech. Rep. INT-141. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 83 p. [923]
23. Fonda, R. W. 1979. Fire resilient forests of Douglas-fir in Olympic National Park: a hypothesis. In: Linn, Robert M., ed. Proceedings, 1st conference on scientific research in the National Parks, Vol. 2; 1976 November 9-12; New Orleans, LA. NPS Transactions and Proceedings No. 5. Washington, DC: U.S. Department of the Interior, National Park Service: 1239-1242. [6698]
24. Garrison, George A.; Bjugstad, Ardell J.; Duncan, Don A.; [and others]. 1977. Vegetation and environmental features of forest and range ecosystems. Agric. Handb. 475. Washington, DC: U.S. Department of Agriculture, Forest Service. 68 p. [998]
25. Gleason, Henry A.; Cronquist, Arthur. 1991. Manual of vascular plants of northeastern United States and adjacent Canada. 2nd ed. New York: New York Botanical Garden. 910 p. [20329]
26. Great Plains Flora Association. 1986. Flora of the Great Plains. Lawrence, KS: University Press of Kansas. 1392 p. [1603]
27. Haeussler, S.; Coates, D.; Mather, J. 1990. Autecology of common plants in British Columbia: A literature review. Economic and Regional Development Agreement FRDA Rep. 158. Victoria, BC: Forestry Canada, Pacific Forestry Centre; British Columbia Ministry of Forests, Research Branch. 272 p. [18033]
28. Haeussler, S.; Pojar, J.; Geisler, B. M.; [and others]. 1985. A guide to the interior cedar-hemlock zone, northwestern transitional subzone (ICHg), in the Prince Rupert Forest Region, British Columbia. Land Management Report Number 26; ISSN 0702-9861. Victoria, BC: British Columbia, Ministry of Forests. 263 p. [6930]
29. Hagle, Susan K.; McDonald, Geral I.; Norby, Eugene A. 1989. White pine blister rust in northern Idaho and western Montana: alternatives for integrated management. Gen. Tech. Rep. INT-261. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 35 p. [9357]
30. Halpern, Charles B.; Harmon, Mark E. 1983. Early plant succession on the Muddy River mudflow, Mount St. Helens, Washington. American Midland Naturalist. 110(1): 97-106. [8870]
31. Hamer, David; Herrero, Stephen; Brady, Keith. 1991. Food and habitat used by grizzly bears, Ursus arctos, along the Continental Divide in Waterton Lakes National Park, Alberta. Canadian Field-Naturalist. 105(3): 325-329. [18672]
32. Hamilton, Evelyn H.; Yearsley, H. Karen. 1988. Vegetation development after clearcutting and site preparation in the SBS zone. Economic and Regional Development Agreement: FRDA Report 018. Victoria, BC: Canadian Forestry Service, Pacific Forestry Centre; British Columbia Ministry of Forests and Lands. 66 p. [8760]
33. Hickman, James C., ed. 1993. The Jepson manual: Higher plants of California. Berkeley, CA: University of California Press. 1400 p. [21992]
34. Hitchcock, C. Leo; Cronquist, Arthur. 1973. Flora of the Pacific Northwest. Seattle, WA: University of Washington Press. 730 p. [1168]
35. Hulten, Eric. 1968. Flora of Alaska and neighboring territories. Stanford, CA: Stanford University Press. 1008 p. [13403]
36. Humphrey, Harry B.; Weaver, John Ernst. 1915. Natural reforestation in the mountains of northern Idaho. Plant World. 18: 31-49. [12448]
37. Keller, Marilyn Crane. 1980. Post-fire recovery within ravine forest communities of Pattee Canyon, Missoula, Montana. Missoula, MT: University of Montana. 136 p. Thesis. [6725]
38. Kovalchik, Bernard L.; Hopkins, William E.; Brunsfeld, Steven J. 1988. Major indicator shrubs and herbs in riparian zones on National Forests of central Oregon. R6-ECOL-TP-005-88. Portland, OR: U.S. Department of Agriculture, Forest Service, Pacific Northwest Region. 159 p. [8995]
39. Kramer, Neal B.; Johnson, Frederic D. 1987. Mature forest seed banks of three habitat types in central Idaho. Canadian Journal of Botany. 65: 1961-1966. [3961]
40. Kuchler, A. W. 1964. Manual to accompany the map of potential vegetation of the conterminous United States. Special Publication No. 36. New York: American Geographical Society. 77 p. [1384]
41. La Roi, George H.; Strong, Wayne L.; Pluth, Donald J. 1988. Understory plant community classifications as predictors of forest site quality for lodgepole pine and white spruce in west-central Alberta. Canadian Journal of Forest Research. 18: 875-887. [5414]
42. Lyon, L. Jack. 1971. Vegetal development following prescribed burning of Douglas-fir in south-central Idaho. Res. Pap. INT-105. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 30 p. [1495]
43. Lyon, L. Jack; Stickney, Peter F. 1976. Early vegetal succession following large northern Rocky Mountain wildfires. In: Proceedings, Tall Timbers fire ecology conference and Intermountain Fire Research Council fire and land management symposium; 1974 October 8-10; Missoula, MT. No. 14. Tallahassee, FL: Tall Timbers Research Station: 355-373. [1496]
44. Moss, Virgil D.; Wellner, Charles A. 1953. Aiding blister rust control by silvicultural measures in the western white pine type. Circular No. 919. Washington, DC: U.S. Department of Agriculture. 32 p. [12262]
45. Mueggler, Walter F. 1965. Ecology of seral shrub communities in the cedar-hemlock zone of northern Idaho. Ecological Monographs. 35: 165-185. [4016]
46. Norton, H. H.; Hunn, E. S.; Martinsen, C. S.; Keely, P. B. 1984. Vegetable food products of the foraging economies of the Pacific Northwest. Ecology of Food and Nutrition. 14(3): 219-228. [10327]
47. Noste, Nonan V.; Bushey, Charles L. 1987. Fire response of shrubs of dry forest habitat types in Montana and Idaho. Gen. Tech. Rep. INT-239. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 22 p. [255]
48. Offord, H. R.; Van Atta, G. R.; Swanson, H. E. 1940. Chemical and mechanical methods of Ribes eradication in the white pine areas of the western states. Tech. Bull. No. 692. Washington, DC: U.S. Department of Agriculture. 50 p. [1795]
49. Oswald, E. T.; Brown, B. N. 1993. Vegetation development on skid trails and burned sites in southeastern British Columbia. Forestry Chronicle. 69(1): 75-80. [20566]
50. Padgett, Wayne George. 1981. Ecology of riparian plant communities in southern Malheur National Forest. Corvallis, OR: Oregon State University. 143 p. Thesis. [14933]
51. Pfister, Robert D. 1974. Ribes L.--currant, gooseberry. In: Schopmeyer, C. S., tech. coord. Seeds of woody plants in the United States. Agric. Handb. 450. Washington, DC: U.S. Department of Agriculture, Forest Service: 720-727. [1877]
52. Piper, Jon K. 1986. Seasonality of fruit characters and seed removal by birds. Oikos. 46: 303-310. [15348]
53. Raunkiaer, C. 1934. The life forms of plants and statistical plant geography. Oxford: Clarendon Press. 632 p. [2843]
54. Roland, A. E.; Smith, E. C. 1969. The flora of Nova Scotia. Halifax, NS: Nova Scotia Museum. 746 p. [13158]
55. Saunders, Jack K., Jr. 1955. Food habits and range use of the Rocky Mountain goat in the Crazy Mountains, Montana. Journal of Wildlife Management. 19(4): 429-437. [484]
56. Sawyer, John O.; Thornburgh, Dale A. 1977. Montane and subalpine vegetation of the Klamath Mountains. In: Barbour, Michael G.; Major, Jack, eds. Terrestrial vegetation of California. New York: John Wiley & Sons: 699-732. [685]
57. Shiflet, Thomas N., ed. 1994. Rangeland cover types of the United States. Denver, CO: Society for Range Management. 152 p. [23362]
58. Singer, Francis J. 1979. Habitat partitioning and wildfire relationships of cervids in Glacier National Park, Montana. Journal of Wildlife Management. 43(2): 437-444. [4074]
59. Soper, James H.; Heimburger, Margaret L. 1982. Shrubs of Ontario. Life Sciences Misc. Publ. Toronto, ON: Royal Ontario Museum. 495 p. [12907]
60. Stark, N. 1983. The nutrient content of Rocky Mountain vegetation: a handbook for estimating nutrients lost through harvest and burning. Misc. Publ. 14. Missoula, MT: University of Montana, School of Forestry, Montana Forest and Conservation Experiment Station. 81 p. [8617]
61. Steele, Robert; Geier-Hayes, Kathleen. 1989. The grand fir/mountain maple habitat type in central Idaho: succession and management. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 148 p. Review draft. [8435]
62. Stickney, Peter F. 1980. Data base for post-fire succession, first 6 to 9 years, in Montana larch-fir forests. Gen. Tech. Rep. INT-62. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Forest and Range Experiment Station. 133 p. [6583]
63. Stickney, Peter F. 1985. Data base for early postfire succession on the Sundance Burn, northern Idaho. Gen. Tech. Rep. INT-189. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 121 p. [7223]
64. Stickney, Peter F. 1989. Seral origin of species originating in northern Rocky Mountain forests. Unpublished draft on file at: U.S. Department of Agriculture, Forest Service, Intermountain Research Station, Fire Sciences Laboratory, Missoula, MT; RWU 4403 files. 7 p. [20090]
65. Strausbaugh, P. D.; Core, Earl L. 1977. Flora of West Virginia. 2nd ed. Morgantown, WV: Seneca Books, Inc. 1079 p. [23213]
66. Strong, W. L.; Pluth, D. J.; LaRoi, G. H.; Corns, I. G. W. 1991. Forest understory plants as predictors of lodgepole pine and white spruce site quality in west-central Alberta. Canadian Journal of Forest Research. 21: 1675-1683. [17695]
67. U.S. Department of Agriculture, Natural Resources Conservation Service. 2018. PLANTS Database, [Online]. U.S. Department of Agriculture, Natural Resources Conservation Service (Producer). Available: https://plants.usda.gov/. [34262]
68. U.S. Department of the Interior, National Biological Survey. [n.d.]. NP Flora [Data base]. Davis, CA: U.S. Department of the Interior, National Biological Survey. [23119]
69. Usui, Masayuki; Kakuda, Yukio; Kevan, Peter G. 1994. Composition and energy values of wild fruits from the boreal forest of northern Ontario. Canadian Journal of Plant Science. 74(3): 581-587. [24583]
70. Vogl, Richard J.; Ryder, Calvin. 1969. Effects of slash burning on conifer reproduction in Montana's Mission Range. Northwest Science. 43(3): 135-147. [8546]
71. Wallmo, Olof C.; Regelin, Wayne L.; Reichert, Donald W. 1972. Forage use by mule deer relative to logging in Colorado. Journal of Wildlife Management. 36: 1025-1033. [4486]
72. Welsh, Stanley L.; Atwood, N. Duane; Goodrich, Sherel; Higgins, Larry C., eds. 1987. A Utah flora. Great Basin Naturalist Memoir No. 9. Provo, UT: Brigham Young University. 894 p. [2944]
73. Yole, D.; Lewis, T.; Inselberg, A.; [and others]. 1989. A field guide for identification and interpretation of the Engelmann spruce-subalpine fir zone in the Prince Rupert Forest Region, BC. Victoria, BC: Ministry of Forests, Research Branch. 81 p. [17095]
74. Zager, Peter Edward. 1980. The influence of logging and wildfire on grizzly bear habitat in northwestern Montana. Missoula, MT: University of Montana. 131 p. Dissertation. [5032]
75. Zamora, Benjamin Abel. 1975. Secondary succession on broadcast-burned clearcuts of the Abies grandis - Pachistima myrsinites habitat type in northcentral Idaho. Pullman, WA: Washington State University. 127 p. Dissertation. [5154]
76. Zamora, Benjamin A. 1982. Understory development in forest succession: an example from the Inland Northwest. In: Means, J., ed. Forest succession and stand development research in the Inland Northwest; [Date of conference unknown]; [Location of conference unknown]. Corvallis, OR: Oregon State University, Forest Research Lab: 63-69. [8766]
77. Fischer, William C.; Bradley, Anne F. 1987. Fire ecology of western Montana forest habitat types. Gen. Tech. Rep. INT-223. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 95 p. [633]
78. Rowe, J. S. 1983. Concepts of fire effects on plant individuals and species. In: Wein, Ross W.; MacLean, David A., eds. SCOPE 18: The role of fire in northern circumpolar ecosystems. Chichester; New York: John Wiley & Sons: 135-154. [2038]
79. Wenger, Karl F., editor. 1984. Forestry handbook. 2d ed. New York: John Wiley & Sons. 1335 p. [8996]